The 400 year old shark does not exist: it is 392 plus or minus 120, and nobody has rechecked it
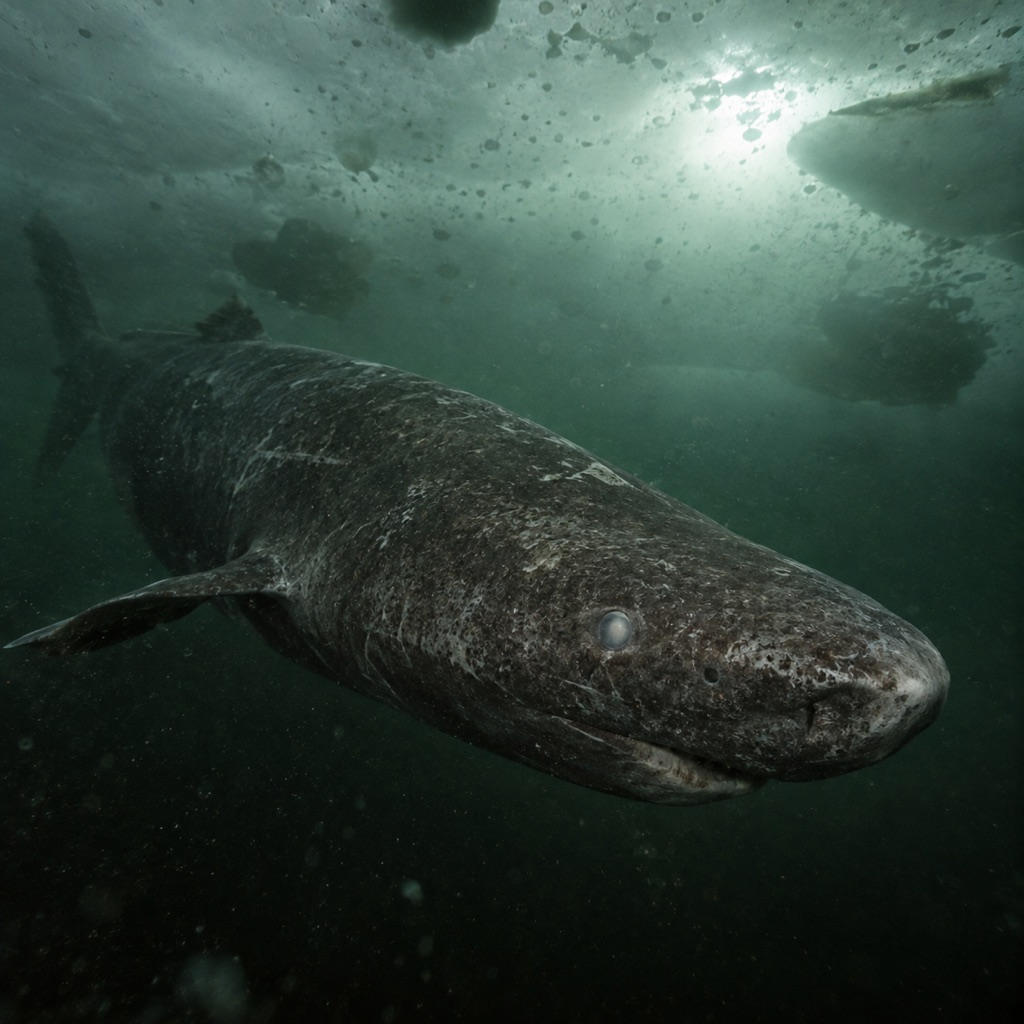
A Greenland shark hauled up in a trawl tells you nothing about its age. Its teeth are replaced continuously, its skeleton is cartilage, and it has no otolith, that inner ear concretion whose layers are counted in bony fish. For decades, the biology of the species was written without its most elementary figure. In the issue dated 12 August 2016, Science published an answer with numbers in it, from a team with Julius Nielsen as first author, obtained by radiocarbon dating the lens nucleus of twenty eight females.
What everyone thought was impossible
The line has been going around for a long time: you cannot age a shark, because it has no otoliths. Taken as a general rule, the line is wrong. Sharks are aged by counting the pairs of bands laid down in the vertebral centra, and the method has been validated in certain species. Steven Campana, Lisa Natanson and Sigmund Myklevoll showed in 2002 that the vertebral bands of the porbeagle do record one year each, at least up to 26 years (Canadian Journal of Fisheries and Aquatic Sciences, vol. 59, pp. 450 to 455). The same paper reports the opposite for the shortfin mako: the methods then in use gave incorrect ages. Validation therefore holds species by species, never wholesale.
The Greenland shark's problem is narrower and more brutal: the species has no usable calcified tissue, which rules out any chronology based on growth zones. The one number the literature held on to about its growth came from a tagging programme followed by recaptures, run in Greenland and published by P. M. Hansen in 1963 in the special publications of the International Commission for the Northwest Atlantic Fisheries (no. 4, pp. 172 to 175): annual growth of 1 centimetre or less. For an adult of 400 to 500 centimetres, the arithmetic suggested something unusual without demonstrating anything.
And band counting gets it wrong, including where it was thought to be reliable. In 2014, Li Ling Hamady, Lisa Natanson, Gregory Skomal and Simon Thorrold radiocarbon dated the vertebrae of eight white sharks from the northwest Atlantic: about 40 years for the largest female (526 centimetres fork length), about 73 years for the largest male (493 centimetres), where earlier counts had topped out between 12 and 23 years (PLOS ONE, vol. 9, no. 1, e84006).
An archive sealed inside the eye
The idea of dating a vertebrate through its eye did not begin with sharks. In 1987, Jeffrey Bada, Christian Vrolijk, Stephen Brown, Ellen Druffel and Robert Hedges published a note in Geophysical Research Letters (vol. 14, no. 10, pp. 1065 to 1067) titled "Bomb radiocarbon in metabolically inert tissues from terrestrial and marine mammals", measuring radiocarbon in two tissues that are never renewed: the lens nucleus of a monkey and a narwhal tusk.
In 1999, John George, Jeffrey Bada, Judith Zeh and their coauthors applied a similar logic to the bowhead whale, analysing 48 eyeballs by aspartic acid racemisation. Four individuals, all of them males, came out above one hundred years (Canadian Journal of Zoology, vol. 77, no. 4, pp. 571 to 580).
The cleanest demonstration came from human anatomy. On 30 January 2008, Niels Lynnerup, Henrik Kjeldsen, Steffen Heegaard, Christina Jacobsen and Jan Heinemeier published in PLOS ONE (vol. 3, no. 1, e1529) the analysis of 13 lenses taken from 13 deceased people. The conclusion: the crystallins of the lens nucleus are formed for the most part around the time of birth, and whatever is added afterwards stays very small and keeps shrinking. The gap between the predicted year of birth and the real one held under three years, with a mean uncertainty of 1.5 years at 95 percent confidence. Jan Heinemeier, of the AMS centre in Aarhus, is also an author on the 2016 shark paper.
The bomb peak, an accidental clock
The marker that makes any of this datable is a geopolitical accident. Atmospheric tests of thermonuclear weapons injected carbon 14 into the atmosphere from the middle of the 1950s onward. The Treaty Banning Nuclear Weapon Tests in the Atmosphere, in Outer Space and Under Water was signed in Moscow on 5 August 1963 and entered into force on 10 October 1963 (United Nations Treaty Series, vol. 480, no. 6964). The reference compilation by Quan Hua and his coauthors places the atmospheric maximum in 1963 and 1964 for the northern hemisphere, in 1964 and 1965 for the southern hemisphere (Radiocarbon, vol. 64, no. 4, pp. 723 to 745).
That signal then works its way down into the ocean, and from there into the food webs. By overlaying marine chronologies of both inorganic and dietary origin, Nielsen and his coauthors show that the onset of the peak in the North Atlantic is synchronous to within a few years and no later than the start of the 1960s. That date is the fixed point everything else hangs on.
Twenty eight females, from 81 to 502 centimetres
The sample comes from scientific surveys carried out in Greenland between 2010 and 2013: 28 females, from 81 to 502 centimetres in total length. The terminal date of the analysis is set at 2012, since collection was spread over three years. Measurements are expressed as a percentage of modern carbon, and the stable isotopes of carbon and nitrogen serve to check where the carbon came from. The result of that check matters: the isotopic signature of the embryonic nucleus is dietary in origin and corresponds to a high trophic level, which is to say it reflects the mother's diet, not that of the animal caught. The chronology also rests on an assumption the authors state outright: size and age are positively correlated.
The distribution is clear cut. The two smallest individuals are above 99 percent modern carbon: they carry the mark of the peak, so they were born after it appeared, at the start of the 1960s, without any precise age being attachable to them. The third, 220 centimetres long, comes in at 95.06 percent, just above the other twenty five, which all stay below 95 percent. The authors therefore give it about 50 years as of 2012 and classify the twenty five larger animals as predating the peak.
For those, the measurement alone is not enough: the natural marine radiocarbon curve varies little across the last four centuries, and the depletion of surface waters differs from one region to the next. The authors calibrate with the Marine13 curve and the OxCal 4.2 software, inside a Bayesian model constrained by von Bertalanffy growth, size at birth, the fixed age of shark no. 3 and plausible reservoir offsets. The model returns an asymptotic length of 546 centimetres with a standard deviation of 42, consistent with the largest individuals ever measured, and an overall agreement index of 109.6 percent. A sensitivity analysis shifts the date of the peak's onset from 1958 to 1980 without overturning the conclusion.
What 392 years actually means
Ages are given as the midpoint of the 95.4 percent probability interval, together with the half range of that interval. Shark no. 28, at 502 centimetres, comes out at 392 years plus or minus 120. No. 27, at 493 centimetres, at 335 years plus or minus 75. Since females are held to reach maturity beyond 400 centimetres, the age at first reproduction is put at a minimum of 156 years plus or minus 22, based on no. 19, measured at 392 centimetres.
The lifespan of "at least 272 years" quoted in the abstract is not a separate measurement: it is, to the digit, the lower bound of the interval for the largest individual, 392 minus 120. It is the hardest claim in the set to argue with, and it is the one the authors put forward.
Two independent lines of evidence point the same way. Sharks under 300 centimetres come out at less than one hundred years, which is indirectly corroborated by the depletion of their carbon 13, something the authors cautiously tie to the Suess effect from fossil fuels. The loads of man made contaminants suggest, for their part, that females of around 300 centimetres are past 50 years. The order of magnitude also stays plausible among living things: the authors recall that the bowhead whale is credited with about 211 years, and that the ocean quahog, a bivalve, reaches 507 years. That last comparison proves nothing; it locates.
One thing the paper does not supply has to be added: validation by a second method. In 2019, a collective review published in Frontiers in Marine Science (vol. 6, article 87), cosigned by four authors of the 2016 study, states that these estimates still need to be verified by an independent dating technique that is both precise and accurate, and that the pathway and residence time of bomb radiocarbon into deep Arctic waters and into the shark's prey remain poorly known.
Why the short version won
On 11 August 2016, the day before the issue date, Science ran a news piece by Elizabeth Pennisi titled "Greenland shark may live 400 years, smashing longevity record" (DOI 10.1126/science.aag0748). The slippage takes two moves: 392 rounds up to 400, and the plus or minus 120 disappears. What is left is a round number with no margin, easier to repeat than the real structure of the result, which is a Bayesian interval resting on a single fixed point.
The value of the work is not the record, though. It lies in the age at maturity: a species that does not breed before a century and a half of life will not rebuild its numbers on the timescale of a management plan. The Greenland shark is a common bycatch of Arctic and subarctic demersal fisheries, and it has been the target of attempts at commercial exploitation. In 2015, the Norwegian red list, the one the authors cite, classified it as data deficient.
Ten years on, that number is still the one people quote. The chromosome level genome assembly for the species, posted in the Proceedings of the National Academy of Sciences on 19 May 2026 (vol. 123, no. 21, e2601272123), runs to 5.9 billion bases for an N50 of 233 megabases and a completeness of 96.7 percent, and its abstract recalls the 2016 estimate in its second sentence: 392 years plus or minus 120. Citing is not retesting. Ten years later, the interval has not been narrowed by a second method; it has been copied.